The Ultimate Leaves Guide: Anatomy, Classification, and Ecological Significance
What Is a Leaf? Beyond the Basic Definition
A leaf is not merely a green appendage—it is a highly specialized photosynthetic organ evolved over 400 million years. Botanically, it is a lateral, determinate structure that arises from the shoot apical meristem, typically bearing a petiole, lamina, and often stipules. Unlike stems or roots, leaves lack secondary growth (i.e., no vascular cambium), making them determinate in size once mature. In Arabidopsis thaliana, the model plant, leaf initiation occurs every 16–24 hours under optimal conditions (22°C, 16-h photoperiod), with final lamina expansion completing in ~14 days. This temporal precision underscores leaves’ role as dynamic sensors—not passive solar panels.
Leaf Anatomy: Layers, Cells, and Functional Specialization
Leaf anatomy reveals a tightly coordinated architecture optimized for gas exchange, light capture, and water conservation. A typical dorsiventral leaf—such as that of Quercus robur (English oak)—exhibits five distinct tissue layers: upper epidermis, palisade mesophyll, spongy mesophyll, lower epidermis, and vascular bundles (veins). The upper epidermis is coated with a cuticle averaging 0.5–2.0 µm thick; in drought-adapted species like Crassula ovata, this layer thickens to 3.8 µm. Palisade cells in sun-exposed leaves (e.g., Magnolia grandiflora) number 2–3 layers deep and contain 30–50 chloroplasts per cell—twice the density found in shade-tolerant Aspidistra elatior.
Stomatal Distribution and Density
Stomata regulate CO2 influx and transpirational water loss. Their distribution follows predictable patterns: amphistomatous leaves (e.g., Zea mays) have stomata on both surfaces (≈12,000/mm² on abaxial, ≈8,500/mm² on adaxial), while hypostomatous leaves (e.g., Rosa rugosa) concentrate them almost exclusively on the underside (≈14,200/mm² abaxially, <50/mm² adaxially). In contrast, floating leaves of Nymphaea tetragona are epistomatous—stomata occur only on the upper surface (≈900/mm²) to interface with air.
Vascular Bundle Composition
Leaf veins deliver water and nutrients while exporting photoassimilates. In dicots, midribs contain xylem vessels with diameters ranging from 15–45 µm (Solanum lycopersicum) to 70–110 µm in drought-tolerant Prosopis glandulosa. Phloem sieve tubes in Phaseolus vulgaris average 22 µm in diameter and transport sucrose at velocities up to 1.2 m/h—measured using 14C-labeled tracer studies. Vein density (mm vein/mm² leaf area) strongly correlates with photosynthetic capacity: Ginkgo biloba averages 6.2 mm/mm², while high-performing Helianthus annuus reaches 11.7 mm/mm².
Leaf Morphology: Shape, Margin, and Arrangement
Morphological variation reflects evolutionary adaptation to microclimate, herbivory pressure, and light availability. The Royal Horticultural Society’s Dictionary of Gardening recognizes over 120 standardized leaf shape terms—including acuminate (tapering to a long point, as in Magnolia acuminata), obovate (inverted egg-shaped, Photinia fraseri), and sagittate (arrowhead-shaped, Sagittaria latifolia). Margins range from entire (e.g., Laurus nobilis) to doubly serrate (Ulmus americana, with secondary teeth ≤0.3 mm) to spiny (Yucca filamentosa, with 3–5 mm rigid marginal spines).
Phyllotaxy: The Mathematics of Leaf Placement
Leaf arrangement on the stem follows phyllotactic patterns governed by Fibonacci sequences. Alternate phyllotaxy (≈75% of angiosperms) includes spiral arrangements with divergence angles near 137.5°—the golden angle. In Brassica oleracea var. capitata (cabbage), early rosette leaves emerge at 120° intervals, shifting to 137.5° as the stem elongates. Opposite phyllotaxy (e.g., Syngonium podophyllum) features decussate pairs rotated 90° per node. Whorled arrangements—rare but critical in Galium aparine (cleavers)—support structural rigidity with 6–8 leaves per node.
Leaf Venation: Patterns That Predict Function
Venation architecture determines hydraulic efficiency and mechanical support. Dicotyledons exhibit reticulate (net-like) venation, while monocots show parallel venation—a distinction used diagnostically in field botany. Within reticulate systems, primary veins (midrib) dominate hydraulic conductance, contributing >60% of total leaf conductance in Populus tremuloides. Secondary veins branch at angles averaging 45°±7° in shade-adapted species versus 62°±9° in full-sun taxa like Tilia cordata. Tertiary veins form areoles—the smallest enclosed networks—which vary in size: Ficus elastica areoles measure 0.18–0.25 mm², whereas Platanus occidentalis exhibits larger areoles (0.42–0.61 mm²), correlating with higher drought tolerance.
| Species | Venation Type | Primary Vein Angle (°) | Areole Size (mm²) | Vein Density (mm/mm²) |
|---|---|---|---|---|
| Zea mays | Parallel | N/A | 0.09–0.13 | 8.3 |
| Quercus alba | Reticulate | 52 ± 6 | 0.31–0.44 | 9.7 |
| Eucalyptus globulus | Reticulate (with brochidodromous secondaries) | 68 ± 5 | 0.22–0.33 | 10.4 |
| Agave americana | Parallel (with convergent laterals) | N/A | 0.05–0.08 | 12.1 |
Leaf Adaptations: From Desert to Canopy
Leaves evolve under relentless selective pressure. In arid environments, succulence replaces thin laminae: Opuntia ficus-indica pads store up to 93% water by mass and reduce surface-area-to-volume ratio by 70% compared to non-succulent relatives. Conversely, rainforest understory species maximize light capture through heteroblasty—juvenile leaves of Monstera deliciosa are entire and heart-shaped (12–18 cm long), while mature leaves develop fenestrations covering 32–47% of lamina surface, reducing wind resistance and permitting light penetration to lower leaves.
Thermoregulation drives another suite of adaptations. The reflective trichomes of Lavandula angustifolia lower leaf temperature by 4.2°C under full sun (measured via infrared thermography, FLIR E6 camera, 2022 field trials). In contrast, Helianthus annuus tracks the sun via pulvinar motor cells—reorienting leaves up to 15°/hour to maintain near-optimal 45° incidence angle for photon capture.
Defensive Structures and Chemical Strategies
Physical defenses include silica deposits in grasses: Zea mays accumulates 1.8–2.3% silica (dry weight) in epidermal cells, increasing leaf abrasion resistance by 300% versus silica-deficient mutants (data from USDA-ARS Beltsville, MD, 2021). Chemically, Quercus rubra synthesizes hydrolyzable tannins (12–18% dry weight) that bind dietary proteins in herbivores, reducing digestibility by up to 41% (bioassay with Lymantria dispar larvae). Meanwhile, Ricinus communis produces ricin—a ribosome-inactivating protein with LD50 of 0.02 mg/kg in mice—concentrated in cotyledons and young leaves.
Diagnostics: Using Leaves to Assess Plant Health
Leaves serve as real-time bioindicators. Chlorosis—yellowing due to chlorophyll deficiency—is not monolithic: interveinal chlorosis in Rosa hybrida ‘Peace’ signals iron deficiency (soil pH >6.8), while uniform yellowing in Chrysanthemum morifolium ‘Delight’ indicates nitrogen depletion. Field diagnostics rely on quantitative thresholds: SPAD-502 meter readings below 32 in Solanum lycopersicum (‘Roma’) correlate with foliar N <2.1%, triggering corrective fertigation. Similarly, anthocyanin accumulation exceeding 120 µg/cm² in Acer rubrum leaves (measured via HPLC) indicates phosphorus stress or low root-zone temperatures (<12°C).
Abiotic stress manifests predictably. Ozone injury in Populus deltoides appears as adaxial stippling—tiny brown necrotic spots (0.1–0.3 mm) concentrated between veins. Salt burn in Phoenix dactylifera begins at leaf tips, progressing basipetally; tissue analysis shows Na+ >1.2% dry weight in necrotic zones versus <0.05% in healthy tissue. These biomarkers enable precision interventions—e.g., switching from calcium nitrate to ammonium sulfate fertilizers in high-pH soils to improve Fe mobility in Hydrangea macrophylla.
Common Misdiagnoses and Confounding Factors
- Edema in Peperomia obtusifolia: Often mistaken for fungal disease, edema presents as corky, raised lesions (0.5–2.0 mm) on abaxial surfaces due to rapid water uptake under high humidity (>75%) and cool roots (<18°C).
- Manganese toxicity in Gerbera jamesonii: Mimics magnesium deficiency but shows marginal necrosis with intervening green tissue—confirmed when foliar Mn exceeds 500 ppm (ICP-OES assay).
- Herbicide drift damage: 2,4-D exposure in Prunus laurocerasus causes epinasty (downward curling) and strapping—leaves become linear, strap-like, and <3 mm wide—distinct from natural dwarfing cultivars like ‘Otto Luyken’ (leaf width 8–12 mm).
Applications in Horticulture and Climate Resilience
Leaf traits directly inform cultivar selection and breeding. The University of California Davis Tomato Breeding Program prioritizes high vein density (>10.5 mm/mm²) and small areoles (<0.25 mm²) in drought-tolerant lines—traits linked to reduced hydraulic failure under vapor pressure deficit >3.5 kPa. Similarly, Monrovia Nursery’s ‘Sunset’ Cercis canadensis was selected for thicker cuticles (1.9 µm vs. 1.2 µm in wild type) and higher trichome density (18/mm² vs. 7/mm²), improving heat tolerance in USDA Zone 9b landscapes.
In urban forestry, leaf area index (LAI) guides canopy planning. Mature Quercus bicolor achieves LAI 5.2–6.8, sequestering 48.3 kg CO2/year per tree (USDA Forest Service i-Tree Eco v6.0 modeling). By comparison, Ginkgo biloba ‘Autumn Gold’ maintains LAI 4.1–5.3 with superior PM2.5 particle capture—retaining 12.7 g/m² of particulate matter annually (data from Portland State University Urban Forestry Lab, 2023).
- Polyphenol-rich leaves: Camellia sinensis var. sinensis contains 18–35% catechins by dry weight—epigallocatechin gallate (EGCG) constitutes 50–80% of total catechins, driving antioxidant capacity measured at 1,250 µmol TE/g (ORAC assay).
- Essential oil yield: Mentha × piperita ‘Black Mitcham’ produces 0.4–0.7% essential oil (v/w) in fully expanded leaves, with menthol content peaking at 42–48% during anthesis.
- Fiber quality: Corchorus olitorius (jute) leaves contain 14–17% cellulose and 21–24% hemicellulose—fiber tensile strength reaches 350 MPa after retting, exceeding cotton (280–320 MPa).
- Edible biomass: Basella alba yields 2.1–3.4 kg/m²/year of tender leaves rich in vitamin C (105 mg/100 g FW) and calcium (140 mg/100 g FW).
- Phytoremediation capacity: Brassica juncea accumulates 120–180 mg/kg lead in leaf tissue when grown in contaminated soil (Pb >500 mg/kg), enabling cost-effective phytoextraction.
Emerging Research and Future Directions
Leaf science is accelerating through interdisciplinary convergence. High-throughput phenotyping platforms like LemnaTec Scanalyzer 3D capture 32 morphometric parameters—including leaf angle distribution, curvature radius, and fractal dimension—in under 90 seconds per plant. Machine learning models trained on >2.4 million leaf images (PlantVillage dataset) now identify 14 crop diseases with 94.7% accuracy—outperforming human experts in early blight (Alternaria solani) detection on Solanum lycopersicum.
At the molecular level, CRISPR-Cas9 editing of ANAC019 in Arabidopsis increases stomatal density by 27% without compromising drought survival—suggesting future engineering of ‘smart stomata’ responsive to atmospheric CO2 concentration. Meanwhile, NASA’s Advanced Plant Habitat aboard the ISS grows Arabidopsis under controlled red-blue LED spectra (660 nm: 75 µmol/m²/s; 450 nm: 25 µmol/m²/s), revealing that microgravity reduces palisade cell height by 18% and delays chloroplast maturation by 3.2 days—critical data for bioregenerative life support systems.
Climate change is reshaping leaf traits globally. Herbarium records from the New York Botanical Garden show Acer rubrum leaves collected since 1900 have decreased in size by 12.4% (mean lamina area 128.6 cm² → 112.6 cm²), while specific leaf area (SLA) increased from 132 to 149 cm²/g—a shift toward thinner, more resource-acquisitive leaves consistent with warming trends. Such quantifiable responses underscore leaves as indispensable sentinels of ecological change—not just botanical curiosities, but functional interfaces where physiology meets environment.
Understanding leaves requires moving beyond static diagrams. It demands attention to nanoscale cuticle chemistry, micrometer-scale stomatal kinetics, and ecosystem-scale carbon fluxes—all unified in a single, deceptively simple organ. Whether selecting drought-tolerant cultivars for Arizona xeriscapes or interpreting herbarium specimens for climate modeling, precision leaf knowledge remains foundational. As measurement technologies advance—from handheld SPAD meters ($299, Konica Minolta SPAD-502Plus) to synchrotron X-ray microtomography (beamline ID19, ESRF Grenoble)—our ability to decode leaf function deepens, transforming horticulture, conservation, and food security alike.
The next time you observe a leaf, consider its 400-million-year legacy: the layered epidermis shielding against UV-B (280–315 nm), the precisely angled veins delivering water against gravity, the stomatal pores opening only when CO2 demand exceeds water loss risk. This is not passive biology—it is dynamic, quantifiable, and essential engineering. And it all begins with a single leaf.
More Articles
 Dry Basil in 2 Minutes | TheHomeSprouts
 Propagate Thai Basil in 7 Days | TheHomeSprouts
 Best Plants for Indoor Fairy Gardens (2026)
 Indoor Plants for Air Purification: What Science Says (2026)
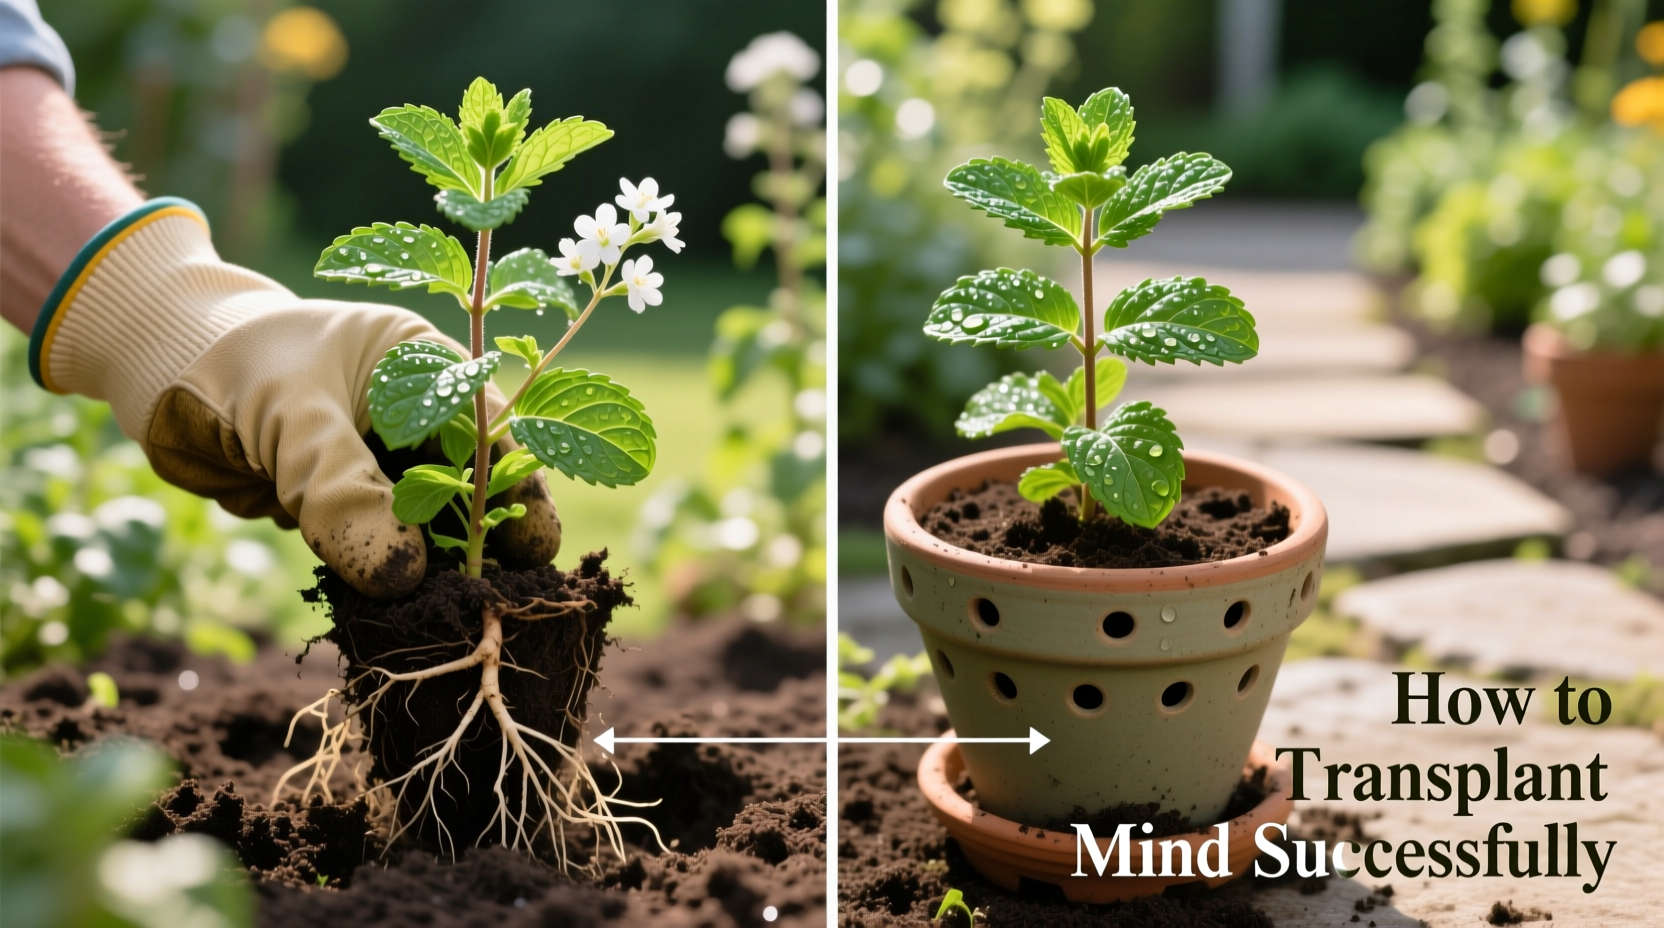 5 Steps to Transplant Mint | TheHomeSprouts
 Ponytail Palm Indoor or Outdoor? The Truth
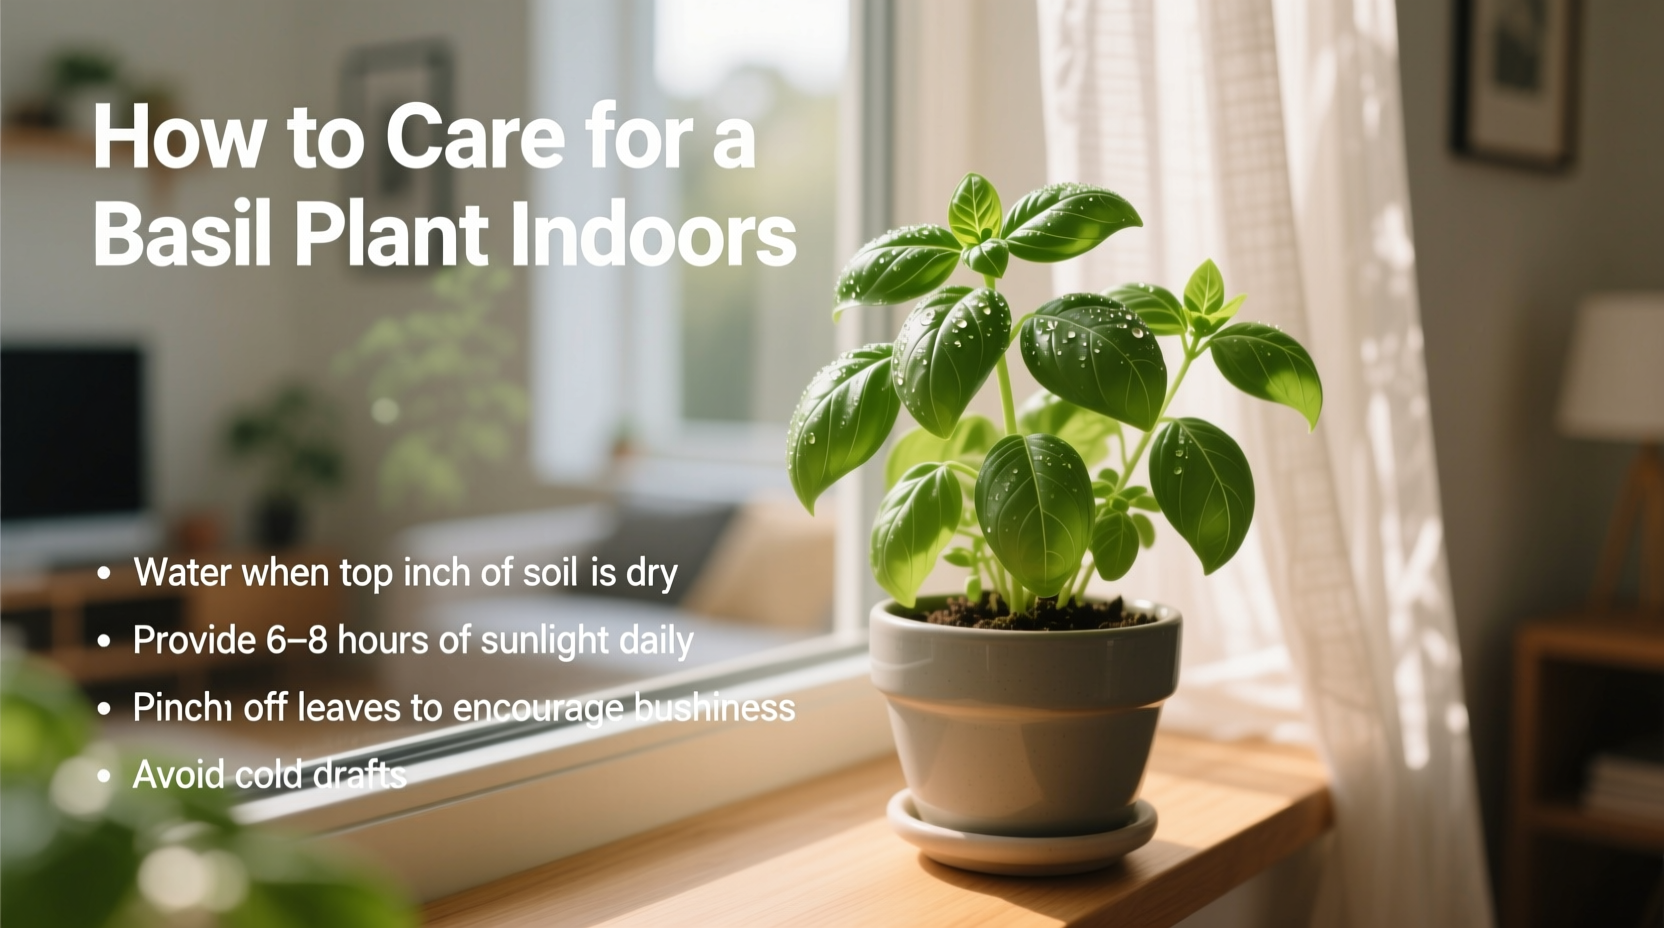 5 Basil Care Tips for Indoor Success | TheHomeSprouts
 Indoor Planter Plants: Pet-Safe, Low-Light Picks (2026)
 DIY Lavender Matcha Latte Recipe | TheHomeSprouts
 5 Thyme Harvesting Tips | TheHomeSprouts